Paul Smith on the Cambrian Explosion
Listen to the podcast here or wherever you get your podcasts.
-
This transcript was generated automatically and lightly edited for readability.
Oliver Strimpel: This is Geology Bites with Oliver Strimpel. We've all heard of the Cambrian explosion of life, a time when the nature and number of life forms changed rapidly during the early to middle Cambrian. The explosion is documented by the appearance of a profusion of animal fossils in some Cambrian beds, perhaps most famously in the Burgess Shale in the Canadian Rocky Mountains. Many fossils from this period are kept for preservation, research and display in natural history museums. One such museum is the Oxford University Museum of Natural History. Paul Smith is the director of this museum and professor of natural history at Oxford University. In his research, he uses paleobiology, sedimentology and geochemistry to probe the interactions of Earth systems and organisms from the late Neoproterozoic to the Ordovician, a period that spans the Cambrian explosion. Paul Smith, welcome to Geology Bites.
Paul Smith: Thank you for inviting me.
Oliver Strimpel: What exactly do we see in the fossil record that tells us there was such rapid diversification of life in the Cambrian that we call it an explosion?
Paul Smith: We geologists call the period of geological time from the Cambrian through to the Recent the Phanerozoic, and that gives the game away, really. The etymology of that term is visible life, or visible animals. So in the lower part of the Cambrian, we begin to see a profusion of animal fossils of many different groups, and evolution then proceeds through the Phanerozoic to the modern day. Initially the Cambrian was defined as being the appearance of the first fossils. Now we define it by the appearance of the traces of the first complex animals, and that's a little bit lower than it was traditionally placed. But really, in the broadest terms, it reflects the emergence of abundant animals within oceanic ecosystems.
Oliver Strimpel: In a previous episode of Geology Bites, Rachel Wood talked about the emergence of complex life in the Ediacaran, the period immediately preceding the Cambrian. How many of the developments that we see in such profusion in the Cambrian actually started in the Ediacaran?
Paul Smith: Yeah, that's an interesting question. The last five years have really seen a revolution in our understanding of the Ediacaran-Cambrian transition. It was a problem that Darwin recognized, actually, when he was talking about the Cambrian. He realized that the appearance of the first fossils was not just the appearance of one or two species, but the appearance of a diverse range of species and of diverse body plans, diverse groups. And that suggested to him, bright man, that evolution must have been proceeding for some time and that the evolutionary origin of animals must sit some way underneath their first appearance in the fossil record. And it really perplexed him. He wrote about it and discussed it with a number of people, but he didn't have the tools to really analyze that problem. And up until, let's say, 10 years ago, it was still really problematic. We knew that multicellular animals first appeared in the late Neoproterozoic, in a period that we now call the Ediacaran, so from about 650 million years through to the base of the Cambrian at 540. But we really didn't know what to do with them. They were just called the Ediacaran biota. They were clearly multicellular. There were many, many different interpretations of what they were.
But then, in that revolution that I referred to, starting a little bit more than five years ago, people began to use different techniques. My colleague Frankie Dunn began to use the techniques that developmental biologists would use to look at how these organisms grew from embryo to adult. And she was able to prove quite conclusively that at least some of these organisms in the Ediacaran biota were indeed primitive animals. Other people tried looking at the traces of biological decay, so-called biomarkers. Cholesterol-related molecules are actually quite robust. And although it's slightly more controversial, there's evidence of cholesteroids, which are unique to animals, in the fossil record at that period. So a number of lines of new evidence were converging on the fact that some, if not most, of the Ediacaran biota were primitive animals, and that some of them were reasonably closely related to modern cnidarians, the group that includes corals and anemones.
So that really began to set the focus of, well, in that case, what's the Cambrian explosion? If the origin of animals is way down in the Ediacaran, 20, 30, 40 million years and even more before the appearance of the first abundant animals, then what is the Cambrian explosion? And I think we've now reconciled that the sudden appearance of diverse body plans is the best definition of the Cambrian explosion. And now we're beginning to piece together the evidence. It's a very multidisciplinary approach, with people who are looking at the chemistry, the geochemistry, the biochemistry, the fossils themselves, but also the environments that they were living in. And it's clear that there is an increasing abundance of evidence as we go through the late part of the Ediacaran, particularly from 550 million years onwards. We begin to get the first burrowers, and then we cross the boundary defined by burrowers, and we begin to get the first body fossils in abundance. So the diversification of animals is perhaps gradational, but there must be some key waymarkers that explain this sudden profusion of a multiplicity of different body plans in the fossil record: the Cambrian explosion.
Oliver Strimpel: Whether it occurred in the Ediacaran or in the early to middle Cambrian, something, as you say, really changed at that time. And so a big question that has occupied you and many researchers is, well, what caused the Cambrian explosion? I know that many hypotheses have been proposed. They include astronomical explanations, ones involving the physical and chemical environment that prevailed during the Cambrian, ecological explanations, and developmental or genetic ones. Let's talk about these and start with the astronomical ones.
Paul Smith: I'd started documenting the whole range of hypotheses that have been proposed post-2000 for the Cambrian explosion, and some patterns began to emerge. The first was that there were a huge number of hypotheses. The second was that a lot of them were individual hypotheses, just a single cause. And the third was that those single causes almost always came from within a discipline. So the astrophysicists were convinced it was astrophysical or astronomical explanations for the Cambrian explosion. Geneticists were convinced it was genetics, geologists were convinced it was geology, et cetera, et cetera. So it began to become clear that maybe there was more to it than this.
So the first thing I did was begin to think about, well, which are the ones that we can exclude in a parsimonious way? We don't need to go for the most complex hypothesis. And it was the astronomic ones that leapt up at that point. One of the astronomic hypotheses that have been suggested was that it was an increase in light availability from the young Sun. The Sun wasn't very young. By 500 million years ago it had had a good 4 billion years of existence. Others had proposed that it was an increased level of cosmic ray bombardment that was perhaps increasing mutation rate. And others had proposed that it was an explosive bolide impact, because, well, don't bolides cause everything? So I think that unless the Earth-bound hypotheses don't provide a satisfactory answer, we don't need to resort to astronomic hypotheses.
And then, as I worked through the list of individual hypotheses, it actually became clear that many of them were interlinked, that there was the potential for a chain of cause and effect. And that set us off looking for feedback loops rather than relying on individual hypotheses. And those hypotheses, once we'd eliminated astronomical ones, largely centered on geological hypotheses, geochemical hypotheses, and then biological or genetic hypotheses.
Oliver Strimpel: Well, let's talk about those. Perhaps you can explain what the line of argument for each of those is first, and then we can talk about how they interact in the feedback loops. So starting with the geochemical and the physical ones, I wonder if these stem from the geological or tectonic configuration of the continents and the shallow seas and the consequent geochemistry.
Paul Smith: To some degree that's true, but I think that what people were looking at were much more enclosed hypotheses. So, for example, it had been proposed that an increase in substrate oxygenation might be responsible for the Cambrian explosion, or that an influx of calcium might be the cause, or an influx of nutrients such as phosphates; or that sea level rise might be the cause, leading to continental flooding; that hydrothermal vents might be responsible; that continental collision might be responsible. Virtually every possible hypothesis had been proposed by this stage, including one of my favorites: that supercontinent amalgamation might have led to it, but also that supercontinent breakup might have led to it. So there were even diametrically opposed hypotheses. But within that there were some clear linkages that might be understandable if you viewed it as a series of processes that were interlinked rather than as stand-alone hypotheses.
Oliver Strimpel: How does the geological configuration affect the chemical, then? You mentioned supercontinents and the breakup of supercontinents, which presumably affect how much shallow ocean there is and erosion rates. Is that the connection?
Paul Smith: Yeah, that's exactly right. So we do know that during the later parts of the Proterozoic, the Neoproterozoic, there had been an extensive period where continents had been denuded. There were extensive peneplains formed by erosion to the point of flatness, and we can see that in the rock record. That's well evidenced and well documented. So it doesn't then require much of a sea level rise to flood very far into the interiors of these peneplaned continents. We know that a supercontinent called Rodinia was breaking up at about that time, leading to the formation of lots of new ridges. New ridges have high volumes; they subside as they cool. And when we have periods of enhanced plate spreading, we do know that that's associated in the rock record with sea level rise. It's one of the foundational bases of sequence stratigraphy.
So we know that at the base of what we call Series 2 of the Cambrian, there is a major sea level rise across America. It's a thing called the Great Unconformity, where Cambrian rocks sit on much older crystalline basement, and we see a version of that on many other continental blocks globally. So there certainly is a sea level rise. And the thought was that maybe that sea level rise and continental flooding led to the rapid erosion of the regolith that had accumulated (there was no vegetation on land at that time, of course). And so the flooding of the regolith led to a pulse of inorganic species out into the oceans, including calcium and phosphates, which, as we know from any garden pond, are a powerful nutrient.
Oliver Strimpel: Just to be clear, you mentioned that continental rifting or supercontinental breakup resulted in the formation of mid-ocean spreading ridges, which created more oceanic crust. How does that lead to sea level rise?
Paul Smith: So the formation of a new ridge creates a significant projection up from the base of the ocean. The water's got to go somewhere, so it spills over the edges of the continental margins and floods right the way across the cratons.
Oliver Strimpel: What about the hypotheses based on ecological explanations?
Paul Smith: There were a range of biological ones. Some had suggested that the origin of biomineralization might be a cause. Others had suggested that with that sea level rise there was an increase in habitable area, or habitable volume, of shallow seas within the photic zone. And we know from the species-area effect that if you increase the area of a habitat, then you will increase the diversity of that habitat. Others suggested genome patterning: the way that control genes such as homeobox genes, Hox genes, control the orientation of axes in the developing embryo, front to back, side to side, dorsal to ventral, top to bottom. Others had suggested an increase in food web complexity. Others still, the origin of plankton and nekton, swimming organisms. In other words, the ocean ecosystems became three-dimensional. They weren't just ocean-bed ecosystems. And finally, the origin of burrowing. And actually many of those can be linked together.
Oliver Strimpel: So one thing: all these three different categories, if you like, of explanation that we've discussed so far, the astronomical, the geological and geochemical, and the ecological, are environmental factors. And I'm wondering if this particular confluence of circumstances that we saw in the Cambrian arose for the first time at that time, and that therefore that was when all these things would come together and we could then see this proliferation of life.
Paul Smith: Yeah. Because I think we need to have established starting conditions. So I think the geneticists are absolutely right about the developmental patterning that enables bilaterian animals. That's animals with a plane of symmetry down the midline, unlike the corals and anemones that we talked about earlier. Bilaterians have the potential to occupy a lot more habitats, because that bilaterian body plan lends itself to adaptation to a number of these new habitats. So the only abundant burrowers we find in the modern day are bilaterians, and those swimming organisms, with the exception of jellyfish, are bilaterians. So there seems to be an evolvability of bilaterians.
And to take one example, one of the things that we know from the rock record is that we begin to see increasing amounts of burrowing in the late Ediacaran, going through to the Cambrian, as I mentioned earlier. Those burrows must be made by bilaterians. Those organisms might have been engineering their own habitats. Initially, perhaps the ones that could tolerate low oxygen began to burrow, but as they burrowed, they introduced oxygen from seawater into those substrates, and that enabled other organisms to move in. And so in a relatively short space of time, a few million years, we begin to get this new habitat beneath the sediment-water interface being occupied by a wide range of organisms. And the evidence for that is that we've got a wide range of different burrow types. So we know that the origin of burrowing is a major driver, and that is in turn driven by those organisms oxygenating the environment as they went along and evolved into it.
And the same is true of the origin of plankton and nekton. The evolution of the bilaterian body plan enables free swimming in the water column. It's not a million miles away from the same musculature that enables burrowing. And we then seem to see an arms race. It coincides with the origin of biomineralization. The first question to ask is, are those hard parts, those hard tissues, being used for offense or defense? And actually in the geological record, both of them appear pretty much simultaneously, which suggests that there's some sort of evolutionary arms race going on.
The biomineralization itself may well result from that flux of calcium into the oceans. Calcium is a cell toxin. Most cells will try and expel any calcium that gets to the inside. That hypothesis relies on the fact that, well, maybe natural selection then begins to make use of that waste calcium. The calcium is being combined both with carbonate and phosphate. One of the things that we see is that once organisms appear and they have a biomineral, they stick with that biomineral. So some groups use calcium phosphate, others use calcium carbonate. Very few organisms swap over in their evolutionary history, and the use of calcium carbonate and the use of calcium phosphate again appear at the same time. So there's this major biomineralization event that occurs a little bit below that major sea level event. So there's lots of synchronicity.
But I think we can begin to put things in order. The genetic patterning has got to be there as a prerequisite. And in a way it's just sitting in those populations waiting for the right environmental conditions. The sea level rise provides the right environmental conditions, and that then leads to this cascade of feedback loops.
Oliver Strimpel: That's fascinating. So you're saying that even if we had had that particular confluence of environmental circumstances, with maybe the prevalence of shallow seas or the flooding of peneplains and the right temperature and atmospheric conditions and so on, even if that had happened earlier, the genetic evolution might just not have got to the point where these highly interacting processes that you talked about could run away with evolution and then produce the diversity that we see.
Paul Smith: That's where people are going. You can't have either/or; you've got to have both. It's the old, the older evolutionary story of organisms making the most of an environmental event.
Oliver Strimpel: I think you've hinted at it already, but which of these family of hypotheses do you favor?
Paul Smith: I don't favor any, actually. I think that the geological, the geochemical, the ecological and the genetic interlink in a very intricate way to produce this cascade. And I think that we need to view things in a holistic and interdisciplinary way rather than focusing on individual causal factors. I think that's been one of the mistakes that we've made in the past.
Oliver Strimpel: You said earlier that we're coming more and more to the conclusion that the way to define, or the way to characterize, the Cambrian evolution is that at the end of it, we had the fundamental body plans in place that we have then seen throughout history, and that took place even before life emerged from the oceans onto land. Can you outline what those fundamental body plans are?
Paul Smith: Yeah. So if we divide animal life into different groups of evolutionarily related organisms, we can identify high-level groups on the basis of their distinctive body plans. So for example, cnidarians will be characterized by having radial symmetry. It's often modified in different ways, but most of them have radial symmetry. The majority of animals, as I mentioned, have this bilaterian pattern of having symmetrical halves to their body. If we scale down from bilaterians, we begin to see other patterns. So if we take the group that we're most familiar with, ourselves, the vertebrates and their close relatives, the invertebrate chordates are again characterized by having a stiffening rod that runs the length of the organism, and just before the tip of the stiffening rod is where the anus comes out. So there's what's called a post-anal tail. They're bilateral because they're part of the bilaterian group. So there's a nested element to these character sets, and all vertebrates have that basic body plan, from the most primitive, from hagfishes and lampreys, right the way up to elephants and cheetahs and ourselves.
And then if we take another example, the echinoderms, they typically have, excepting the most primitive fossil examples, fivefold symmetry. So we're very familiar with going down to the beach and seeing a five-rayed starfish. Or if we look at the other organisms within the echinoderm group, they will most commonly have a more subtle five-rayed morphology. So that's what I mean by a body plan, sometimes referred to by the German term Bauplan. Once evolved, these body plans are very consistent through time. What we do know is that nearly all body plans, major body plans, had evolved by the end of the Cambrian. Very few are introduced after the end of the Cambrian.
Oliver Strimpel: And why do these particular body plans then last for the hundreds of millions of years that have elapsed since then? I mean, once you form a body plan, is it very hard to change tack, evolutionarily?
Paul Smith: Yeah, they become developmentally stabilized. It's a hot topic in research terms, but it seems to be the case that the development of the organism begins to constrain how evolution can operate on the body plan itself. So, for example, any mutations tend to be fatal mutations rather than ones that can lead to a change in the morphology.
Oliver Strimpel: The Burgess Shale dates from just after this period of rapid diversification, in the middle Cambrian, about 510 million years ago. Does that really incredibly well-preserved fossil assemblage include all of these fundamental body plans?
Paul Smith: Not all of them. It includes a lot of them, but all environments, up to and including the modern day, will determine the organisms that live in them. And we know that there are peculiarities about the Burgess environment. It's relatively deep; it's sitting in quite an anoxic environment. So not all body plans are there. But if we look at the Cambrian as a whole, nearly all of them are there by the end of the Cambrian.
Oliver Strimpel: Are there other sites around the world that epitomize the end of the Cambrian explosion? And maybe put the question another way: if I was going to travel and have a look at a fossil bed that was a really good example of a well-preserved Cambrian explosion bed, where would I go?
Paul Smith: The search for exceptional preservation has been one of the things that's characterized the past 30 or 40 years of paleontology. We've moved away from just describing lots and lots of trilobites and lots and lots of brachiopods to looking for exceptional preservation that preserves soft tissues, sometimes even down to nervous systems, where we can get a lot more data about these organisms. We can extract a lot more morphological characters, and therefore we can build more robust evolutionary trees. It all started with the Burgess Shale, with the work that Whittington and Briggs and Conway Morris and others did, and that led to people looking for other examples of exceptional preservation.
As you suggest, there are two that are really key to the Cambrian explosion debate, and they sit older than the Burgess Shale. The Burgess Shale is about 508 or 509 million years; these sit down at 520. So right at the point where these body plans are beginning to appear in the fossil record. There's one in China, the Chengjiang Biota in the southern part of China, and there's one in the northernmost part of Greenland, facing the Arctic Ocean, which I've worked on: the Sirius Passet locality. They're almost identical ages, and bizarrely, they were found in the same month in 1984.
Oliver Strimpel: And do they all represent shallow marine environments?
Paul Smith: No, they don't. One of the things that's become clear really quite recently is that they're not in the shallowest water. They're mainly shelf edge. And that's true of the Burgess Shale as well, actually, on the edge of a rather precipitous shelf edge. And that begins to open up some interesting questions about what were the controls on the areas in which early animals were evolving and being preserved. These seem to be very oxygen-poor environments. And there's some interesting work that suggests that we might be looking at oxygenated water in the wrong way. Animal tissues are really quite tolerant of low oxygen levels, and it may be that the adaptation to higher oxygen comes later. So we might need to think about these low-oxygen environments as being where animals first evolved.
So they're in moderately deep water, some, in the case of Ediacaran animals, really quite deep water. They are in low-energy environments. There's a suspicion that maybe early animals weren't very good at coping with dynamic substrates, with sand that was moving around in quite a mobile way. They tend to be living below storm wave base, on stable substrates, and well out of the photic zone. So it's not nutrients that are controlling them, because they'd be living in shallower water if they were highly nutrient-dependent. So if they're living in low-oxygen environments, and it's not the nutrient supply that seems to control the distribution, it may be that substrate, needing a stable, perhaps even microbial-mat-covered substrate, is something that's important in these early animal communities and ecosystems.
Oliver Strimpel: I'm struck, though, that when life began to emerge on land, which is such a different set of constraints, you've got to deal with gravity, you've got humidity variations and temperature variations that you don't see in the marine environments. Yet these body plans survived.
Paul Smith: They get adapted, but the body plans themselves are very resilient, and it's the development of a distinctive chordate body plan in the Cambrian that enables vertebrates to become such a dominant force in terrestrial ecosystems 100 million years later. One has to say that arthropods are pretty good at terrestrial ecosystems as well.
Oliver Strimpel: Can you describe some good representatives of the fundamental body plans that emerged at the end of the Cambrian? Well, not at the end of the Cambrian, but during the Cambrian explosion.
Paul Smith: Well, we've talked about echinoderms with their distinctive fivefold symmetry and cnidarians with their radial symmetry, but the things that we would call phyla... The phylum is one of the highest levels of organization within Linnaean classification. Each of those really represents a body plan. If a four-year-old or a five-year-old can recognize something as a different animal, they're probably recognizing body plans at that point. So priapulid worms, annelid worms, et cetera.
Oliver Strimpel: What are you working on at the moment?
Paul Smith: Our work continues looking partly at Sirius Passet in Greenland. I'm really interested in the way that early animals interacted with their environments, using an interdisciplinary approach of geochemistry and paleobiology and anatomy to really understand how these early ecosystems were constructed. And then, since my PhD days, I've always had an interest in the evolutionary origin of vertebrates. And we've got work that's ongoing, in press at the moment, looking at what is the patterning on the tree, what's the acquisition of characters as we work up the tree of early chordates. The nearest large groups to the chordates are the echinoderms and the hemichordates, very, very different body plans. And the Cambrian explosion and those distinctive cases of exceptional preservation give us a real insight into the combinations of characters that were evolving.
Genomics is a really powerful way of constructing the topology of evolutionary trees. When genomics came along 20 or 30 years ago, it threw a lot of the top-level evolutionary trees out of the window. We recognize combinations of organisms that we hadn't really predicted, or that hadn't been well supported. So genomics is really good at patterning the tree, at getting the scaffolding in place. But what genomics can't do, but which paleobiology can, is add the characters onto the basis of those trees. So what is the order that these characters appear in as you go from the separation of echinoderms and vertebrates and chordates up what we call the stem of the chordates, and then, as the different chordate groups branch off, up the stem of the vertebrates? What's the evidence we can extract from the fossil record about the anatomy of those earliest vertebrates?
Oliver Strimpel: Are there any fossils in your museum's collection that you find particularly informative about these questions?
Paul Smith: We've got a very good collection. A colleague of mine called Martin Brasier, who died a few years ago, devoted his life to scouring the world. He was a field addict, a very good field geologist, and he collected the most amazing set of fossils globally. His collection is sitting in the museum, and it's a rich resource. It's one of our most consulted research tools. He hadn't quite finished cataloging it before he passed away. So there are surprises that emerge from those collections that we didn't know were in there. They're in the notebooks, but we haven't pieced it together. So there's a real element of serendipity, as well as this beautifully cataloged and documented field collection.
Oliver Strimpel: And are there any particular species or family of species that you've focused on, particularly through your own research?
Paul Smith: My own research has been focusing on the chordates when I'm not looking at the ecosystem level. I'm particularly interested in the origin of the chordate group, and there's one group actually that we've been looking at recently called the vetulicolians. And these are truly bizarre animals. They've got a mobile tail (we can tell that from the fossils), but they've basically got something that looks like a crisp packet stuck on the front, an open crisp packet stuck on the front. We think they were filter feeders. They were suspension feeders, analogous to modern tunicates, but unlike most modern tunicates, with active propulsion on the other end; many tunicates are either attached or just drift through the ocean water. Some people have said that these things are arthropods, but we've never agreed with that. And we've got a suite of new material from North Greenland, from Sirius Passet. And there's also been lots of good material coming out of Chengjiang, this other deposit I mentioned. And that's enabled us to piece together the position of vetulicolians, which is in press at the moment. So watch this space.
Oliver Strimpel: Paul Smith, thank you very much.
Paul Smith: Thank you.
Oliver Strimpel: To see pictures and illustrations that support this podcast, go to geologybites.com, where you'll also find transcripts and a subject matter index of all the episodes. There you can also give me feedback, which I welcome, as well as sign up to get my emails about new episodes.

As he explains in the podcast, Paul Smith believes that we need to bring diverse research disciplines to bear on the question of life’s explosive proliferation between 541 and 530 million years ago during the Cambrian period. These disciplines include paleobiology, sedimentology, and geochemistry. He suggests that only when sufficiently evolved genetics and conducive environmental conditions coincided could complex feedback loops begin to operate and drive explosive growth in the abundance and diversity of life.
Smith is Director of the Oxford University Museum of Natural History and Professor of Natural History at the University of Oxford. The photo was taken after a day of excavating at Sirius Passet in northern Greenland.
Courtesy of Jan Audun Rasmussen
Podcast Illustrations
Images courtesy of Paul Smith unless otherwise indicated.
Late Neoproterozoic to Early Phanerozoic Time Scale
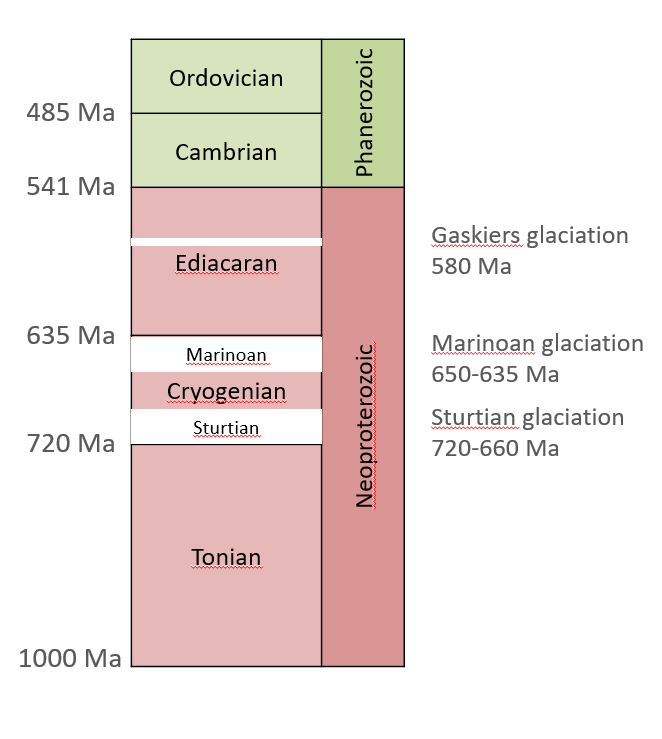
Geological timescale of animal origins. In the two major Snowball Earth glaciations in the Cryogenian period, life survived in limited areas of unfrozen ocean and melt-water ponds on the surface of the ice that covered nearly all the planet. As discussed by Paul Hoffman in his episode of Geology Bites, all modern life is thought to be descended from these organisms. In this episode, Paul Smith talks about the emergence of much more complex life about 100 million years later in the Ediacaran and Cambrian.
Diversification

The major diversification of marine taxa between 635 and 443 million years ago. The red box indicates the time interval discussed in the podcast. EB: Ediacaran biota.
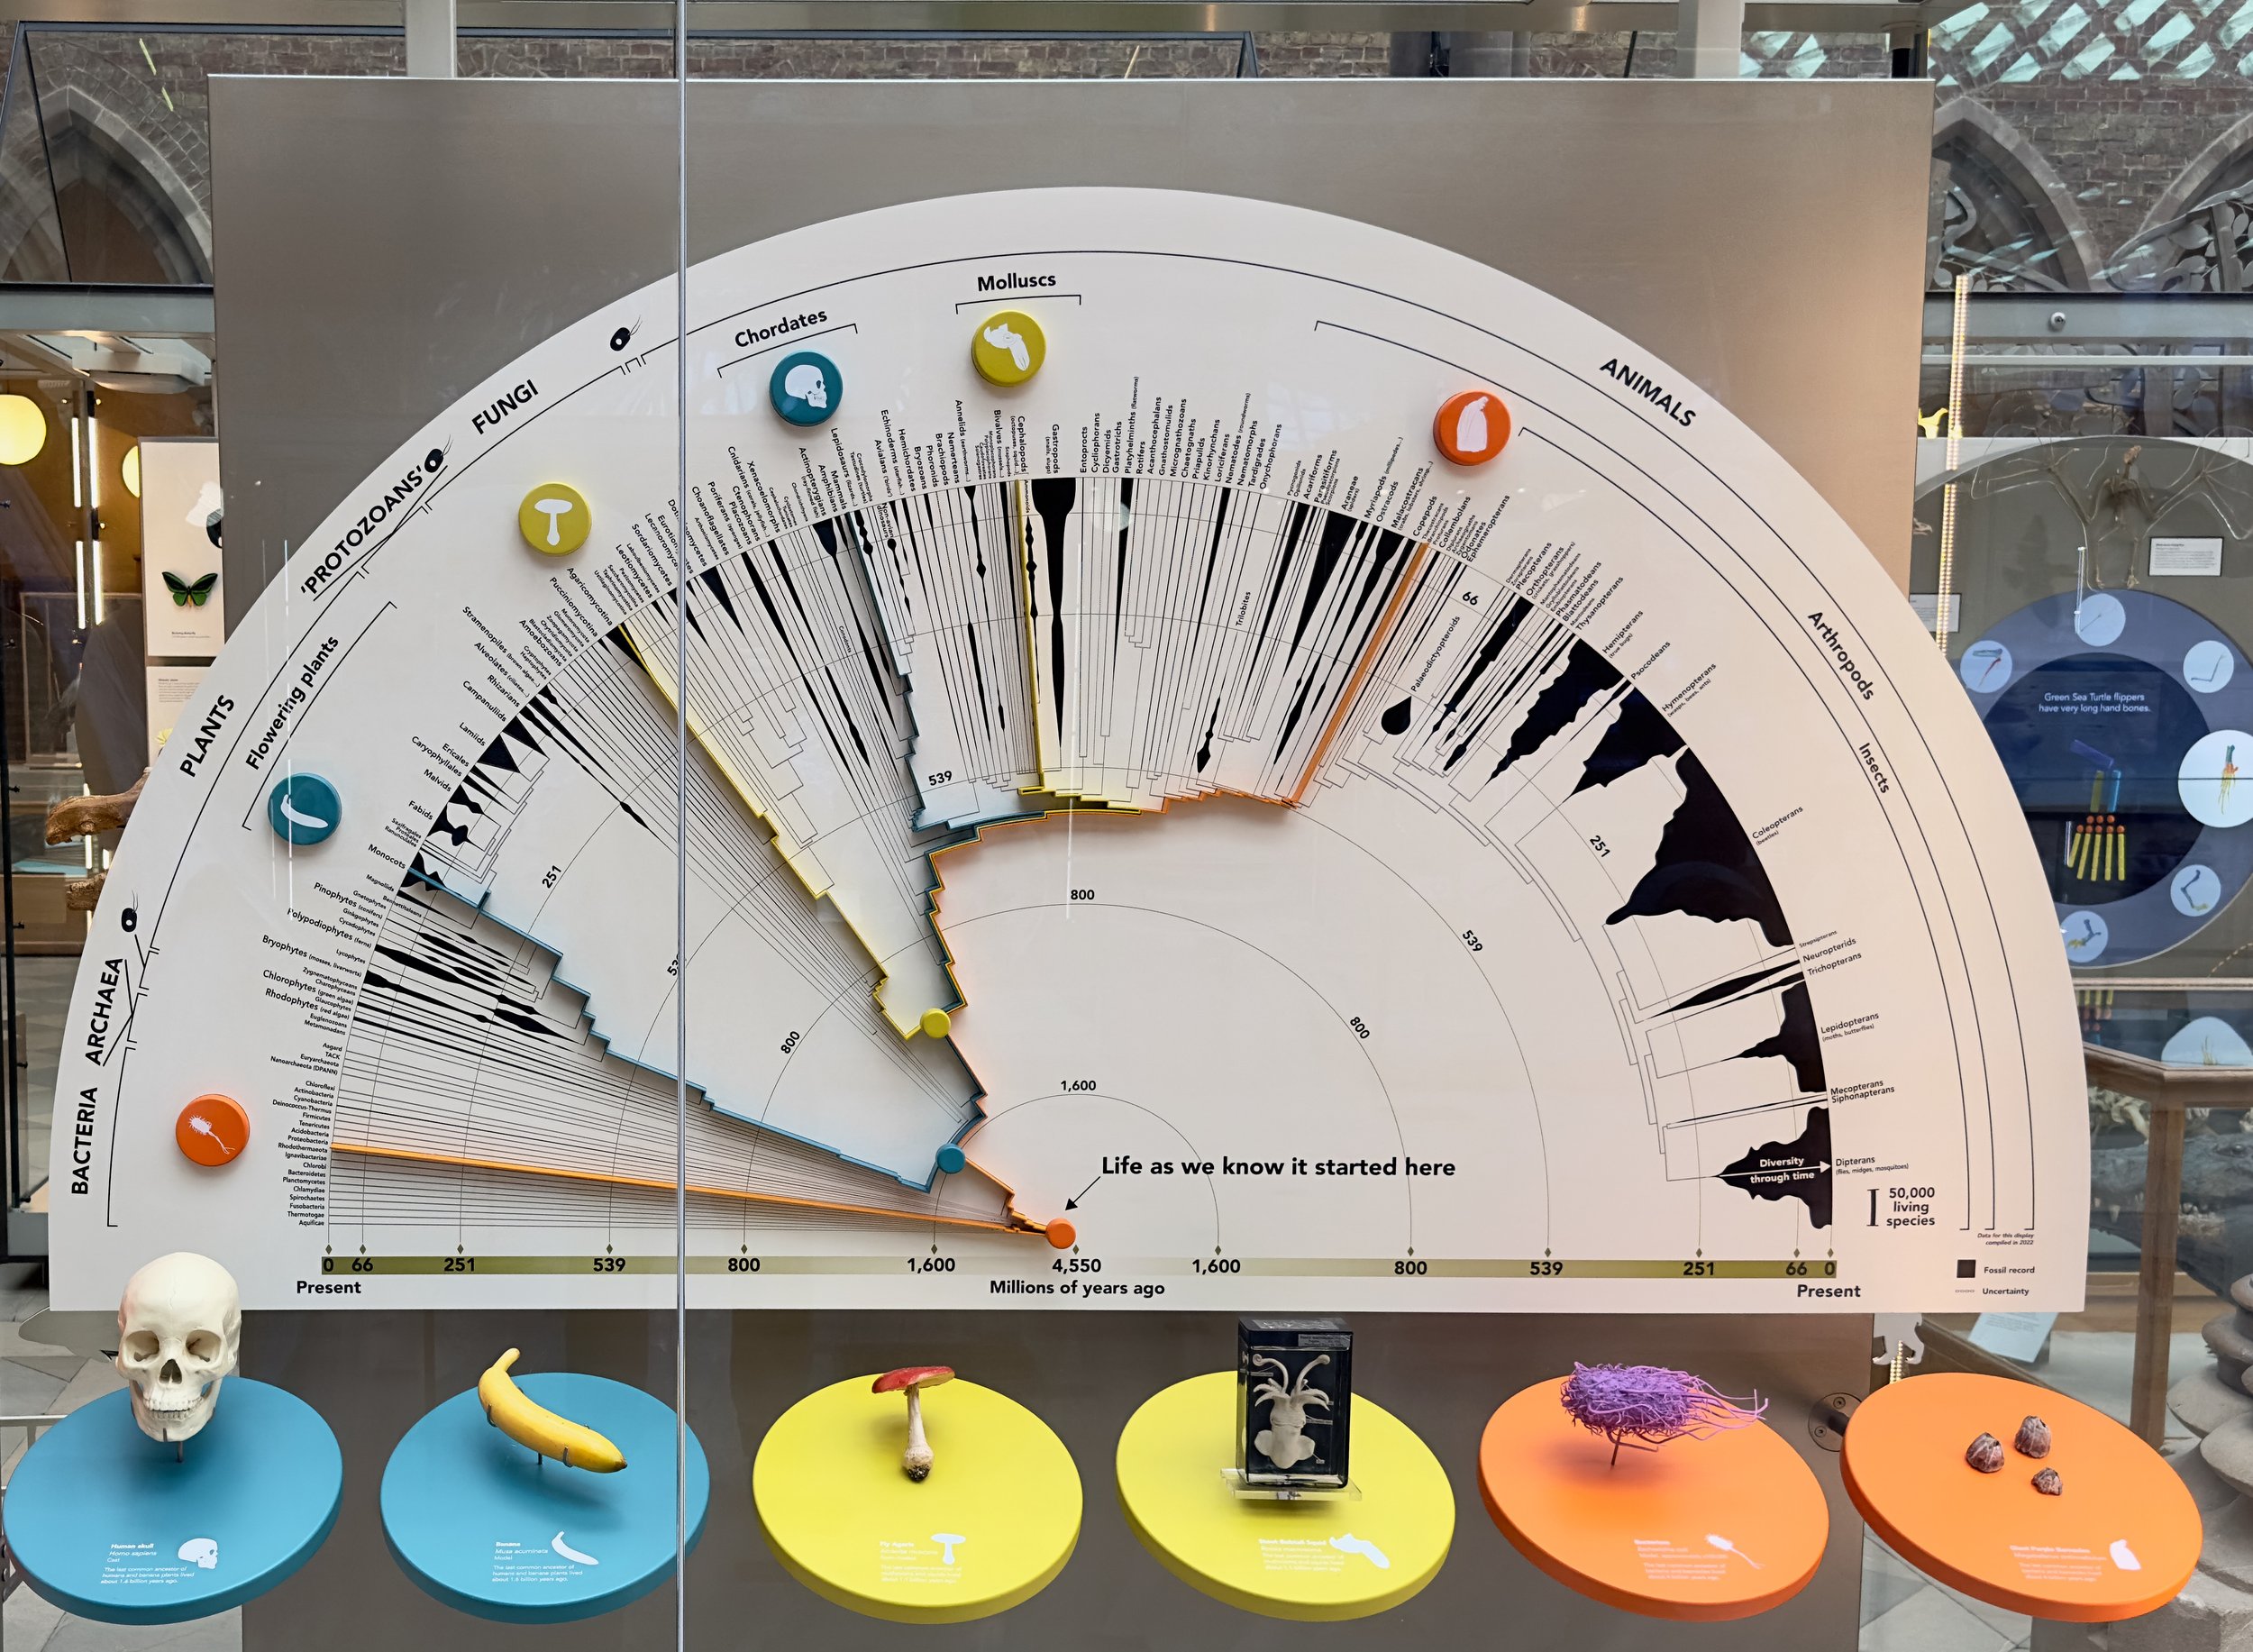
Tree of Life exhibit at the Oxford University Museum of Natural History. Today’s living species are shown at the outermost reaches of the tree. Moving back in time towards the center of the tree, the branching points show the last common ancestor between species. The diversification of the Cambrian explosion appears about halfway to the center (not to scale) just after the divergence of the chordates, molluscs, and arthropods. The tree was constructed using a combination of genetic information, which, as Smith explains in the podcast, provides the scaffolding or framework of the tree, and morphological data from fossils that informs the morphological evolution of groups in their early history. To learn about the evolution of body plans of animal groups that populate the tree of life, we must rely on a combination of genetics and paleobiology.
Interconnected Causes

In the podcast, Smith suggests that no single process is responsible for the Cambrian explosion. Tectonic and geological, developmental, and ecological processes have been hypothesized as isolated, singular causes. Instead, many of these processes are parts of connected feedback loops that together generated the Cambrian explosion. Each box corresponds broadly to a stand-alone hypothesis or suite of related hypotheses (red, geological; blue, geochemical; green, biological). The red arrows connect the explosion in animal diversity to five proximal causes.
The figure represents the interval of time at the beginning of the Cambrian, 541 million to 521 million years ago.
Smith, M.P., et al. (2013), Science 341, 1355
Paleogeography

The configuration of the continents following the breakup of the Rodinia supercontinent about 750 million years ago. The locations of the sites where exceptionally well-preserved beds (Lagerstätten) of Cambrian fossils have been found are marked. Today, the Burgess Shale is in the Canadian Rockies, Sirius Passet is in the far north of Greenland, and Chengjiang is in southern China.
cpgeosystems.com
Burgess Shale

The most famous of the Burgess Shale Formation members at the Walcott Quarry. It dates from 508 million years ago, about 10 million years younger than the Sirius Passet locality. Outcropping at an elevation of 7,500 ft. in the Canadian Rockies, it was discovered by paleontologist Charles Walcott in 1909.
Photo: Mark A. Wilson

Artist’s impression of the deep-water shelf environment where the Burgess Shale biota lived.
Courtesy of D.W. Miller
The Sirius Passet Fossil Bed

Satellite view of North America and Greenland showing the location of Sirius Passet. This location is one of the few known Cambrian Lagerstätten. Their fossils contain preserved soft-tissue structures that provide an important window to the evolution of animals at the time of the Cambrian explosion.
NASA

Geology of the Sirius Passet locality. The fossils lie in the laminated mudstones and muddy siltstones of the Cambrian formation at left. These are bounded at right by a fault where they are in contact with older white carbonate rocks of the uppermost Ediacaran. The fossil quarry site is marked by the red rectangle. At the left end of the rectangle, members of Smith’s team can just be seen.


Left: searching for fossils in the mudstone scree.
Above: preparing the samples for the flight south.

Some of the fauna from the Sirius Passet locality (scale bar = 1 cm). The fauna are dominated by arthropods, some of which lived on the microbial mat surfaces (e.g., a and b left) together with sponges (j) and others in the water column above (e.g., f left, a right). Rarer elements of the fauna include loriciferans (h), palaeoscolecid worms (i), vetulicolians (b right) and polychaete worms (c right).
Harper, D.A.T., et al. (2019), Journal of the Geological Society 176, 1023

As described in the podcast, all the sites of exceptional preservation in the Cambrian appear to have been located at the deep end of a continental shelf where light and nutrients were limited, but where the substrate was stable and free from disturbance by the action of waves and tides. The depositional location of the Sirius Passet Lagerstätte is indicated by a red star.
Harper, D.A.T., et al. (2019), Journal of the Geological Society 176, 1023
Vetulicolians


Left: Vetulicolians from Sirius Passet. The scale bar is 5 cm.
Vinther, J. et al. (2011), Paleontology, 54, 711
Above: artist’s impression of a vetulicolian colony. In the podcast, Smith describes these creatures as having a tail at one end and an open crisp (potato chip) packet at the other.
Courtesy of Katherine Child
Further Reading
Smith, M.P., et al. (2013), Science 341, 1355
Hammerlund, E.U., et al. (2018), Geobiology, 17, 12
Harper, D.A.T., et al. (2019), Journal of the Geological Society 176, 1023
Smith, M.P. (2020) The Cambrian Explosion and the evolutionary origin of animals: Oxford University Museum of Natural History talk: https://www.youtube.com/watch?v=blN-F8n2IAc